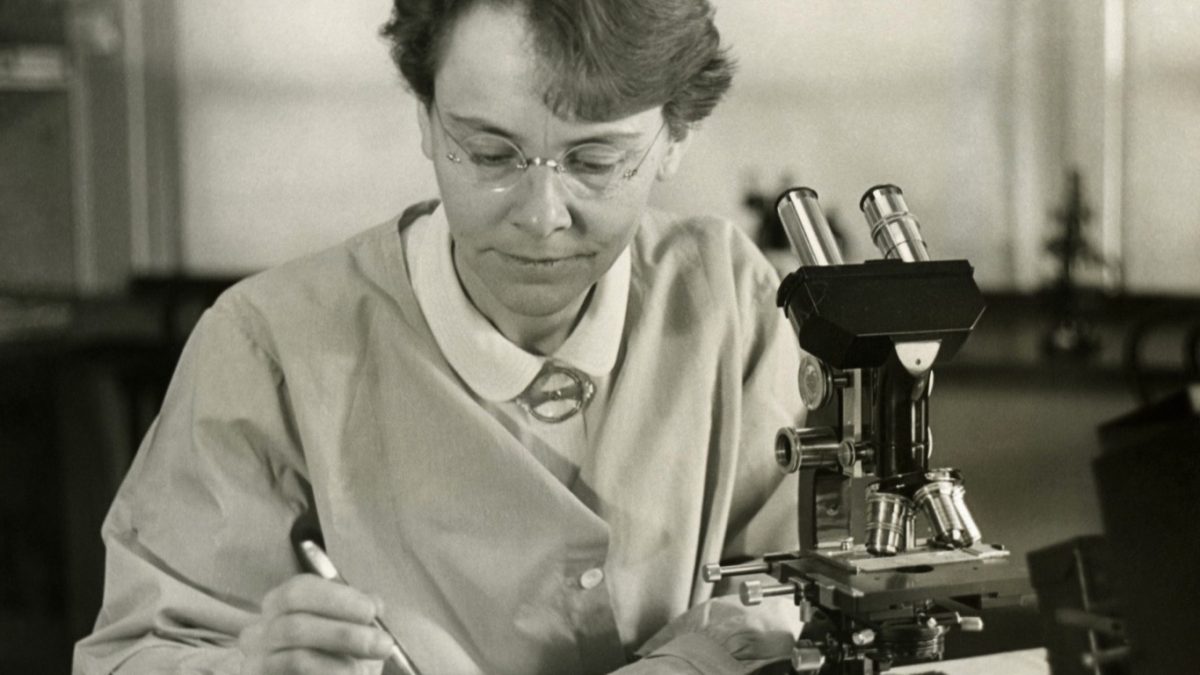
Throughout the first half of the twentieth century, geneticists held an article of faith as unyielding as Newtonian mechanics: The genome is an immutable, static archive. Genes were conceptualized as stationary beads strung permanently upon a chromosomal wire. Mutations could occur, but the physical order of the beads was fixed for eternity. Chromosomes were architectural granite. To challenge this bedrock assumption was considered scientific heresy. Yet in the cornfields of Cold Spring Harbor on Long Island, a solitary cytogeneticist named Barbara McClintock (1902–1992) looked through her monocular microscope and discovered that the genome was alive with restlessness: genes could unmoor themselves, traverse the chromosomal architecture, and jump into entirely new locations.
The Cytogenetics of Zea mays
McClintock was already a legend among cytologists in the 1930s. Working with Indian corn (Zea mays), she had developed exquisite staining techniques to visualize individual maize chromosomes during pachytene of meiosis. In 1931, McClintock and Harriet Creighton had provided the first physical proof of crossing over, correlating cytologically visible chromosomal knobs and translocations with the exchange of genetic markers.
In the mid-1940s, McClintock focused her attention on a puzzling phenomenon: variegation in maize kernels. While normal kernels were uniformly yellow, white, or deep purple, certain mutant ears displayed an erratic, kaleidoscopic mosaic of colored sectors, stripes, and speckles. The size of these colored patches varied wildly—some kernels had tiny dots, others bore large wedges of color. Under classical Mendelian genetics, somatic mutations could not account for such high-frequency, non-random instability occurring repeatedly across thousands of developing endosperm cells.
The Ac-Ds System: Breaking and Jumping
By tracing chromosomal breakage points under the microscope alongside generational breeding records, McClintock identified a specific site on the short arm of chromosome 9 where frequent, spontaneous chromosome breaks occurred. She christened this chromosomal breakage locus Dissociation ($Ds$).
However, McClintock noticed that $Ds$ did not break spontaneously on its own. It required the presence of a second, independent genetic locus, which she termed Activator ($Ac$). When $Ac$ was absent from the genome, $Ds$ was completely stable and immobile. But as soon as $Ac$ was introduced through a cross:
- $Ds$ would induce physical chromosome breakage, shearing off the distal arm of chromosome 9 carrying dominant wild-type genes for brown pericarp and purple aleurone, unmasking recessive colorless alleles.
- More shockingly, $Ds$ could suddenly transpose—vanishing from its original chromosomal position and inserting directly into an adjacent gene (such as the anthocyanin pigment gene $C$).
- When $Ds$ inserted into gene $C$, it disrupted its coding sequence, turning off pigment production (producing a colorless, yellow kernel sector).
- Later in development, in the presence of $Ac$, $Ds$ could spontaneously excise itself from gene $C$ and jump elsewhere, restoring pigment synthesis and creating a vivid purple speckle against a yellow background!
The earlier in kernel development that $Ds$ jumped out, the larger the resulting purple patch. McClintock had discovered Transposable Elements (Transposons)—popularly dubbed “jumping genes.”
“I was startled when I saw that they had moved. It wasn’t just that they moved, but that they exercised control over other genes at the site of integration. I called them controlling elements.”
— Barbara McClintock (1983)
Three Decades in the Wilderness
When McClintock presented her comprehensive data at the Cold Spring Harbor Symposium in 1951, her lecture was met with stony silence, incomprehension, and condescension. Geneticists regarded maize genetics as arcane, and the idea of moving genetic elements threatened the emerging, tidy world of bacterial molecular biology. McClintock chose not to argue: “If you know you are on the right track, if you have this inner knowledge, then nobody can turn you off… no matter what they say.” She ceased publishing her transposon work in mainstream journals, documenting her findings only in the annual Carnegie Institution Year Books.
Vindication arrived in the late 1960s and 1970s, when bacterial geneticists discovered insertion sequences (IS elements) and transposons mediating multi-drug antibiotic resistance in plasmids. Molecular cloning in the 1980s proved that McClintock’s $Ac$ element encoded an enzyme—transposase—that excised the terminal inverted repeats of $Ds$ and pasted it elsewhere via a cut-and-paste mechanism.
When the Human Genome Project was completed, scientists were stunned to discover that transposons and their retroviral evolutionary descendants (LINEs, SINEs, and Alus) constitute nearly half of all human genomic DNA. Transposons were not rare botanical freaks; they were the dynamic tectonic plates of evolutionary novelty, exon shuffling, and genomic regulation. In 1983, at the age of eighty-one, Barbara McClintock received an unshared Nobel Prize in Physiology or Medicine—the ultimate triumph of solitary empirical vision over scientific orthodoxy.