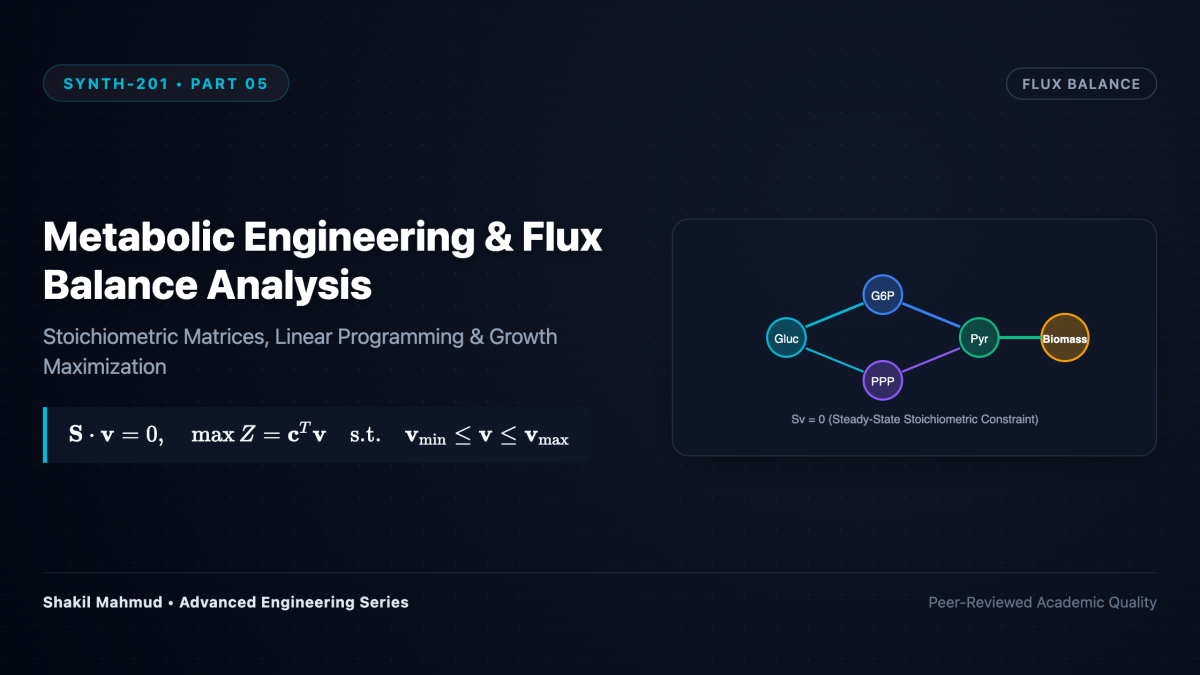
Living cells are chemical micro-refineries, catalyzing thousands of interconnected enzyme reactions simultaneously to convert simple carbon feedstocks into biomass, energy, and secondary metabolites. In Metabolic Engineering, the objective is to rewire this cellular circuit to overproduce high-value molecules—such as pharmaceutical precursors, biofuels, and industrial bioplastics. Because tracking nonlinear kinetic parameters ((K_m, V_{max})) for thousands of enzymes is intractable, researchers rely on constraint-based reconstruction: Flux Balance Analysis (FBA).
1. Genome-Scale Metabolic Models (GEMs) and the Stoichiometric Matrix
Consider a network of (m) metabolites undergoing (n) biochemical reactions. Let (v_j) denote the metabolic flux (rate of reaction (j), typically in ( ext{mmol} cdot ext{gDW}^{-1} cdot ext{hr}^{-1})). The conservation of mass for each metabolite concentration (C_i) is:
[
rac{d C_i}{dt} = sum_{j=1}^n S_{ij} v_j quad iff quad rac{dmathbf{C}}{dt} = mathbf{S} cdot mathbf{v}
]
where (mathbf{S} in mathbb{R}^{m imes n}) is the Stoichiometric Matrix:
- (S_{ij} < 0): Metabolite (i) is consumed in reaction (j).
- (S_{ij} > 0): Metabolite (i) is produced in reaction (j).
- (S_{ij} = 0): Metabolite (i) does not participate in reaction (j).
Because intracellular metabolite turnover occurs on timescales of milliseconds to seconds (( au sim 10^{-3} – 1 ext{ s}))—infinitely faster than cellular doubling times (( au_{ ext{growth}} sim 10^3 – 10^4 ext{ s}))—intracellular metabolite concentrations maintain a dynamic Quasi-Steady State:
[
mathbf{S} cdot mathbf{v} = 0
]
The steady-state flux vector (mathbf{v}) is constrained to lie strictly within the Null Space of the stoichiometric matrix: (mathbf{v} in ker(mathbf{S})).
2. Linear Programming Formulation of Flux Balance Analysis
Because the number of reactions far exceeds the number of metabolites ((n > m)), the null space is underdetermined. To find the biologically realized flux distribution, we superimpose thermodynamic irreversibility and enzyme capacity capacity bounds:
[
v_j^{min} le v_j le v_j^{max}
]
For irreversible reactions, (v_j^{min} = 0); for substrate uptake, (v_{ ext{uptake}}^{max}) is bounded by mass transfer. We then optimize a cellular objective function using Linear Programming (LP):
[
max_{mathbf{v}} Z = mathbf{c}^T mathbf{v}
]
[
ext{subject to: } quad mathbf{S} cdot mathbf{v} = 0, quad mathbf{v}^{min} le mathbf{v} le mathbf{v}^{max}
]
For wild-type organisms evolved under natural selection, the objective vector (mathbf{c}) is chosen to maximize cellular biomass formation: (Z = v_{ ext{biomass}} = mu), where (mu) is the specific growth rate. The biomass equation incorporates the exact stoichiometric proportions of amino acids, nucleotides, lipids, and ATP maintenance required to synthesize one gram of dry cell weight.
3. In Silico Strain Design: OptKnock and Growth-Coupled Production
When synthetic biologists insert a foreign pathway into a microbe to produce a chemical (e.g., 1,4-butanediol or artemisinic acid), the cell naturally downregulates this pathway because foreign product synthesis diverts ATP, NADPH, and carbon away from biomass growth ((max mu)).
To overcome this evolutionary conflict, Burgard, Pharkya, and Maranas formulated OptKnock: a bi-level mixed-integer linear programming (MILP) algorithm that identifies targeted gene knockouts that mathematically force the organism to couple target chemical production directly to its own survival:
[
max_{mathbf{y}} quad v_{ ext{target}}
]
[
ext{s.t.} quad mathbf{v} = argmax_{mathbf{v}^*} left( mathbf{c}^T mathbf{v}^*
ight) quad ext{s.t.} quad mathbf{S}mathbf{v}^* = 0, quad v_j^{min} y_j le v_j^* le v_j^{max} y_j, quad sum (1 – y_j) le K
]
where (y_j in {0, 1}) denotes gene knockout states. In a growth-coupled strain, any cellular mutant that grows faster is mathematically forced to produce more target bioproduct, aligning the relentless force of natural selection with industrial chemical manufacturing.