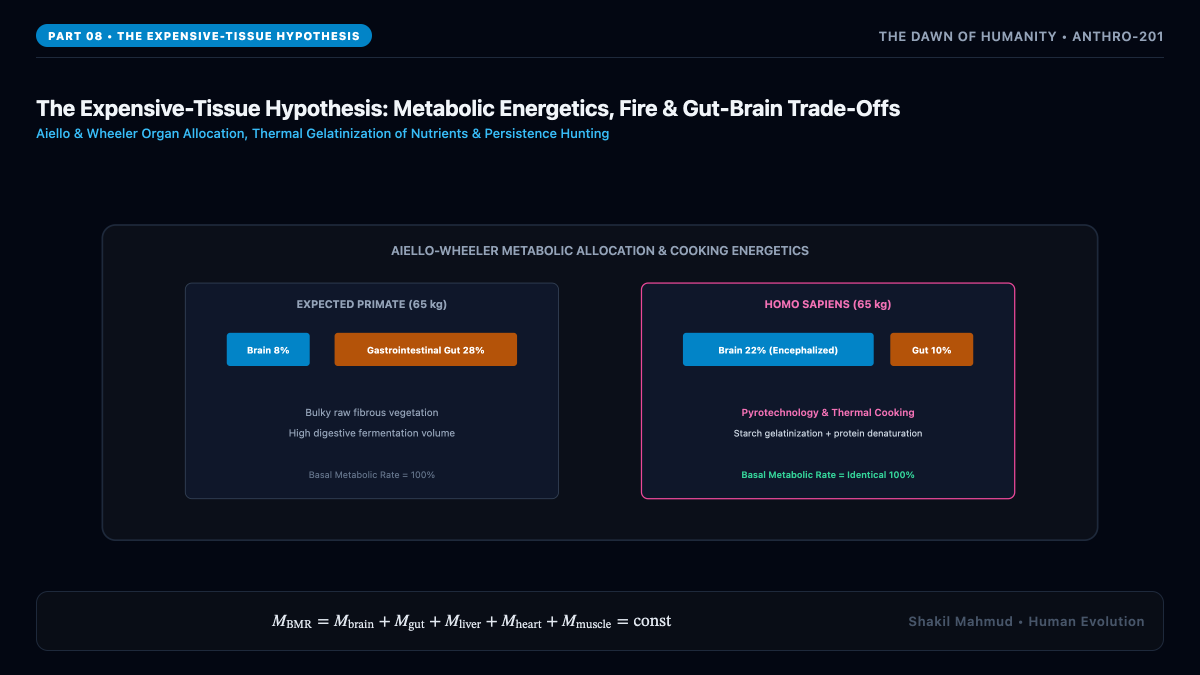
The human brain is an energetic anomaly. Comprising merely $2%$ of an adult’s total body mass, it voraciously consumes more than $20%$ of our total basal metabolic rate (BMR) at rest. In a wild hominin living on the razor’s edge of starvation, sustaining such a metabolically parasitic organ represents an extreme macroevolutionary puzzle. How did early Homo pay the metabolic caloric ransom demanded by runaway encephalization without expanding its overall basal metabolic budget?
1. The Aiello-Wheeler Model: The Metabolic Allocation Equation
In 1995, Leslie Aiello and Peter Wheeler formulated the landmark Expensive-Tissue Hypothesis. In the mammalian body, metabolic energy is not consumed equally by all tissues; it is overwhelmingly monopolized by four “expensive” visceral organs: the brain, the gastrointestinal gut, the liver, and the heart, alongside skeletal muscle mass:
$$M_{text{BMR}} = M_{text{brain}} + M_{text{gut}} + M_{text{liver}} + M_{text{heart}} + M_{text{kidneys}} + M_{text{muscle}}$$
When normalized for organ-specific mass metabolic rates (measured in Watts per kilogram, $text{W/kg}$), brain tissue consumes $approx 11.2text{ W/kg}$ and the gastrointestinal tract consumes $approx 12.2text{ W/kg}$. Together, these visceral tissues demand over $20$ times more energy per gram than resting skeletal muscle ($pprox 0.5text{ W/kg}$).
Crucially, empirical measurements across anthropoid primates reveal that the total basal metabolic rate ($M_{text{BMR}}$) scales with body mass according to Kleiber’s Law ($BMR propto M^{0.75}$), and humans exhibit a BMR virtually identical to that expected for an average primate of our body size. Therefore, encephalization could not be financed by simply elevating total metabolic rate. It had to be paid for by a compensatory reduction in another expensive organ.
Aiello and Wheeler discovered that the human heart, liver, and kidneys are precisely the size expected for a $65text{-kg}$ primate. The only organ that experienced a catastrophic mass reduction was the gastrointestinal tract:
$$Delta M_{text{brain}} = +400% quad longleftrightarrow quad Delta M_{text{gut}} = -60%$$
In herbivorous apes, an enormous fermentation gut (particularly an expanded cecum and colon) is mandatory to host symbiotic cellulose-digesting bacteria capable of fermenting fibrous plant cell walls into short-chain fatty acids (SCFAs). By transitioning to high-quality, calorie-dense, easily digestible foods, early Homo dramatically downsized its gut, releasing the metabolic budget needed to expand the cerebral cortex.
2. The Cooking Hypothesis: Wrangham’s Pyrotechnic Engine
While meat consumption initiated gut reduction in Homo habilis, biological anthropologist Richard Wrangham argued in Catching Fire: How Cooking Made Us Human (2009) that raw meat alone is insufficient to fuel the rapid encephalization of Homo erectus ($900text{–}1,100text{ cm}^3$). Raw meat requires exhausting mechanical mastication (chimpanzees take up to six hours to chew a raw colobus monkey carcass) and exhibits low net metabolizable energy due to the energy expended in digestion (Specific Dynamic Action):
$$E_{text{net}} = E_{text{gross}} – E_{text{digestion}} – E_{text{fecal}} – E_{text{urinary}}$$
Thermal cooking fundamentally alters food chemistry through two universal reactions:
- Starch Gelatinization: Heat causes amylose and amylopectin granules in wild plant tubers to absorb water and swell, destroying their crystalline structure and increasing enzymatic cleavage by salivary and pancreatic amylase from $ 95%$.
- Protein Denaturation: Heat uncoils tightly folded structural proteins (collagen, myosin, actin), exposing peptide bonds to rapid proteolytic cleavage by pepsin and trypsin while softening tough connective tissues.
Cooking acts as external “pre-digestion”, slashing the energy spent on gastrointestinal processing while increasing net caloric yield by $30%$ to $100%$. It simultaneously detoxifies plant secondary compounds and eliminates deadly pathogens.
3. The Archaeological Evidence for Fire Domestication
When did hominins domesticate fire? The archaeological signature of ancient combustion is notoriously elusive due to wind dispersal and post-depositional weathering. The timeline spans several decisive sites:
- Wonderwerk Cave (South Africa, $1.0text{ Ma}$): Micro-stratigraphic Fourier-transform infrared spectroscopy (FTIR) by Francesco Berna and colleagues detected calcined bone fragments and burnt plant ash in sediment layer 10, located $30text{ meters}$ inside the cave where natural lightning could not strike.
- Koobi Fora & Chesowanja (Kenya, $1.5text{–}1.4text{ Ma}$): Thermomagnetic analysis of baked clay clasts indicates heating to $> 400^circtext{C}$, consistent with deliberate campfires.
- Gesher Benot Ya’aqov (Israel, $780text{ ka}$): Spatial clustering of burned flints, wood charcoal, and edible nut species demonstrating habitual, controlled pyrotechnology.
4. Social and Cultural Consequences of the Hearth
The mastery of fire was not merely a nutritional revolution; it remade hominin social structure. By pushing back the nocturnal darkness, fire extended the waking day by four to five hours, shifting social interactions from daytime foraging logistics to nighttime storytelling, social bonding, and cooperative planning. The hearth became the evolutionary cradle of human language, myth, and cultural transmission.