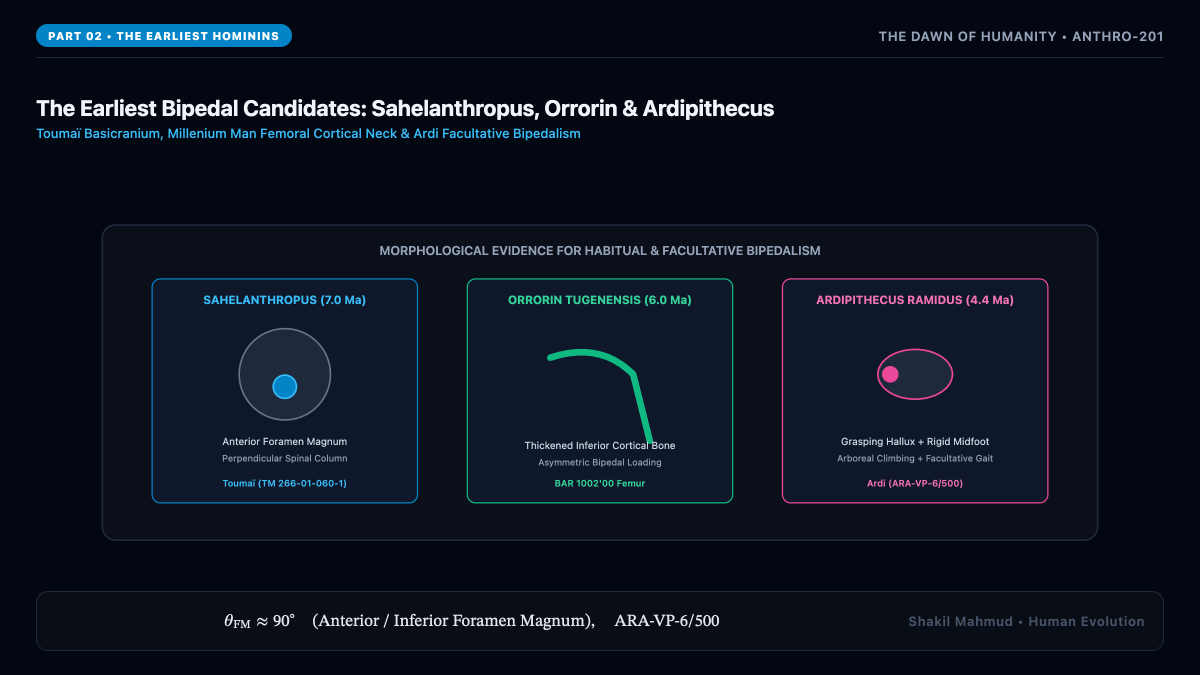
Between seven and four million years ago, the fossil record of African hominoids preserves the tenuous, fragile dawn of the hominin subtribe. Three enigmatic genera—Sahelanthropus from Chad, Orrorin from Kenya, and Ardipithecus from Ethiopia—stand at the evolutionary crossroads, capturing the earliest anatomical experiments in upright bipedal posture while retaining pervasive adaptations for arboreal climbing.
1. Sahelanthropus tchadensis: Toumaï and the Basicranial Revolution ($7.0text{ Ma}$)
In 2001, Michel Brunet and the Mission Paléoanthropologique Franco-Tchadienne (MPFT) discovered a nearly complete, distorted cranium designated TM 266-01-060-1 (popularly dubbed “Toumaï”, meaning “hope of life” in Dazaga) in the Toros-Menalla region of the Djurab Desert in northern Chad. Dated biochronologically and cosmogenically ($^{10}text{Be}/^{9}text{Be}$) to between $7.2$ and $6.8text{ Ma}$, Sahelanthropus fundamentally revised paleoanthropology by demonstrating that early hominin evolution was geographically pan-African rather than confined to the East African Rift Valley.
The hominin status of Toumaï rests upon decisive craniodental apomorphies:
- Position and Angle of the Foramen Magnum: In quadrupeds, the foramen magnum (the aperture through which the spinal cord exits the skull) is situated posteriorly on the occipital planum, orienting the cervical spine horizontally. In Sahelanthropus, the foramen magnum is displaced anteriorly beneath the cranial base. Its basicranial angle with the orbital plane is nearly perpendicular ($pprox 90^circ$), demonstrating that the cranium sat vertically atop an upright, bipedal vertebral column.
- Canine-Premolar Honing Complex ($C/P_3$ Reduction): Modern non-human apes possess an interlocking canine system where large upper canines shear against the lower third premolar ($P_3$), maintaining razor-sharp slicing edges. Sahelanthropus exhibits apical canine wear with no functional $C/P_3$ honing facet, a hallmark hominin reduction in male-male canine display.
2. Orrorin tugenensis: The Millennium Man of the Tugen Hills ($6.0text{ Ma}$)
Discovered in 2000 by Brigitte Senut and Martin Pickford in the Lukeino Formation of the Tugen Hills, Kenya, Orrorin tugenensis ($6.1text{–}5.7text{ Ma}$) provided the earliest postcranial evidence of habitual bipedal locomotion. The hypodigm includes three proximal femoral fragments (specimens BAR 1002’00, BAR 1003’00, and BAR 1215’00).
High-resolution computed tomography (CT) of the BAR 1002’00 femoral neck revealed a defining biomechanical signature of bipedal weight-bearing:
$$text{Cortical Bone Ratio: } frac{text{Inferior Cortical Thickness}}{text{Superior Cortical Thickness}} > 3.0$$
In quadrupedal knuckle-walking apes, the femoral neck experiences symmetrical compressive and bending loads, producing relatively equal cortical bone thickness along the superior and inferior borders ($ ext{ratio} approx 1.0text{–}1.5$). In upright bipeds, cyclical ground reaction forces generate high bending stresses that induce dramatic bone deposition along the inferior margin of the femoral neck. Orrorin possesses a markedly thickened inferior cortex, a long and anteroposteriorly compressed femoral neck, and an obturator externus groove, proving that it habitually bore body weight upright on two hindlimbs.
3. Ardipithecus ramidus: Ardi and Facultative Bipedalism ($4.4text{ Ma}$)
In 1994, Tim White and the Middle Awash project discovered the remarkably complete partial female skeleton ARA-VP-6/500 (“Ardi”) at Aramis in the Afar Depression of Ethiopia. Fully described in 2009, Ardipithecus ramidus presents a profound anatomical mosaic that definitively challenged the century-old assumption that humans evolved from a chimpanzee-like knuckle-walker.
| Anatomical Region | Ardipithecus Morphology | Functional Interpretation |
|---|---|---|
| Pelvis (Innominate) | Broad, short iliac blades with anterior inferior iliac spine (AIIS); lower ischium retains long, ape-like lever arm. | Upper pelvis reconstructed for upright bipedal hip stabilization; lower pelvis retains powerful hamstring lever for climbing. |
| Foot (Pes) | Fully opposable, divergent hallux (big toe); rigid midfoot with plantar os peroneum and cuboid locking. | Tree grasping preserved alongside a rigid lever for terrestrial bipedal push-off without knuckle-walking. |
| Forelimb & Hand | Flexible midcarpal joint; metacarpals lack dorsal ridges; palms flat during quadrupedal arboreal clambering. | Careful arboreal palm-walking (above-branch pronograde clambering); total absence of knuckle-walking specializations. |
| Brain & Dentition | Endocranial volume $sim 300text{–}350text{ cm}^3$; small, blunt canines with reduced sexual dimorphism. | Social structures with diminished male-male physical contest and reduced agonistic canine display. |
Ardi demonstrates that bipedalism did not originate in open, sun-baked savannah grasslands, as hypothesized by Raymond Dart’s classic “savannah hypothesis.” Sedimentology and fossil faunal reconstruction (abundant colobine monkeys and tragelaphin bovids) prove that Ardipithecus lived in closed, wooded canopy environments. Bipedalism evolved as a specialized arboreal/terrestrial facultative foraging adaptation while our ancestors were still deeply anchored in the forest.